Assignment 5.2: Compatible ends
Your answers are saved in this browser. Check them against the downloaded answer key, or open the explanation when you are ready.
Lecture 5.2
Transcript
HAZEL SIVE: From your class exercise about restriction
endonucleases, you should now be able to manipulate
a piece of DNA to reveal blunt ends or sticky ends.
You should know whether or not it's a 5-prime overhang
or a 3-prime overhang.
And this will set us up for the next topic I want to discuss,
which is the question of the vector and ligation.
Let's set the stage for this topic
by looking back at the overall view
that I gave you on cloning and using a gene of interest.
We've talked about cutting the DNA now.
And we haven't talked about how you exactly
isolate your gene of interest.
But we'll not worry about that for the moment.
What we need to talk about now is the next step,
how you're going to put your gene of interest
into some kind of carrier DNA molecule that
will allow it to replicate to high copy number.
And the reason that this can occur
is because of these things called vectors.
A vector is really a virus that grows in bacteria.
It may be pathogenic, or it may be harmless to the bacterium.
The vector is made of DNA.
And it is often circular, in which case
it has got a special name, which is a plasmid.
The trick about plasmids, and any vector,
is that they have something called
an origin of replication.
This is abbreviated ORI.
And this origin in the vector--
I'll write it out--
is an origin of replication.
And this refers to DNA replication.
The origin is a particular sequence
in the plasmid that tells DNA replication to begin.
It is a start site for DNA synthesis.
In fact, it's not just plasmids and vectors
that have got origins of replication.
Our own chromosomes do, too.
I just didn't tell you about them
when we were talking about DNA synthesis.
But now you've heard of them, you
can add that to your compendium of knowledge
about DNA synthesis in general.
This origin of replication allows
the plasmid to replicate within the bacterial host
cell to very high copy number, 10,000 copies or more.
And because you could grow billions and billions
of bacteria without too much difficulty,
you can land up with very large amounts of DNA--
grams, even kilograms of DNA from the right amount
of bacteria that are growing the viral vector.
OK.
So the origin of replication allows the vector
to replicate to something like 10,000 copies per cell.
And that will give you lots of DNA.
There's one other property that vectors usually have.
And that is called a selectable marker,
or two selectable markers.
And I'll tell you what they are in a moment.
But let's just put down that vectors also
have a selectable marker.
There's our vector.
What we have to do now is to insert the gene of interest
into the vector.
We have to do a pasting.
And we paste the gene of interest
into the vector using a particular enzyme called
DNA ligase.
Our gene of interest is pasted, or covalently bonded,
through phosphodiester bonds that
join up the nucleic acid polymer is pasted or covalently bonded
into the vector using an enzyme called DNA ligase.
And just a little note--
you heard about restriction endonuclease and DNA ligase.
If you hear about a molecule that's got the "-ase"
at the end, it's usually an enzyme.
What is this DNA ligase?
It will join together any two compatible DNA ends, OK?
What does that mean?
So ligase joins two compatible DNA ends.
And now, you have to think back to the restriction
endonuclease ends.
Any two blunt ends can be joined together
because there's bluntness there.
There's no kind of nucleic acid hybridization involved.
Any two blunt ends, restriction enzyme endonuclease ends
can ligate.
But the same thing is not true of sticky ends.
There, you've got the single stranded bits sticking out.
That's why they're sticky.
And in order to get sticky ends to ligate,
those sticky single stranded bits
have to base pair with one another.
If they can base pair exactly, then ligase
will join them together and make a covalently closed molecule.
So two complementary, or ends that can base pair,
those complementary ends can ligate.
After ligation of restriction endonuclease cut DNA,
you may or may not regenerate a restriction endonuclease site,
OK?
That's not part of the deal.
So you may or may not regenerate a restriction endonuclease
site.
Let's look at a couple of slides,
so that you can see what I mean.
Here, firstly, is your basic plasmid vector.
This one, called pBR322, was one of the very first
that was used in genetic engineering.
You can see a region called ORI.
That is the origin of replication.
And it's where DNA replication starts.
Both the vector and the gene of interest that you insert in it
will be replicated, starting at this origin of replication.
And then there are these selectable markers
that we mentioned, that are here listed amp and tet.
Now, let's look at some compatible ends.
Any blunt ends can ligate.
I just made up two in the top of the slide.
One of them is half of an SmaI site,
but the other one is a different site.
But they can ligate just fine because all
you need are 3-prime and 5-prime ends to join together.
You need the 3-prime hydroxl and the 5-prime phosphate.
And then ligase can come along.
And it can make a phosphodiester bond between those two
molecules and join them back together again.
Any complementary sticky ends can ligate.
So complementary means that they can base pair.
So for example, in the example of the EcoRI site,
you can see that if you take two 1/2 EcoRI sites
and put them back together again,
that they will be able to ligate and regenerate
a covalently closed DNA molecule and regenerate an EcoRI
site, OK?
The base pairing is exact there.
The AATT on this molecule will base pair
with the TTAA on that molecule.
And you will get out the perfect covalently closed DNA.
On the bottom of the slide, you'll
see that there are two compatible ends there.
They have, again, got the AATT TTAA base
pairing that can make a closed DNA molecule that ligase
can work with.
But in fact, the outcome is not a restriction site.
It's not an EcoRI site.
There is an AT on the 5-prime end of the top strand,
and then the 3-prime end of the bottom strand.
And that doesn't give you an EcoRI site, OK?
So that's some detail about compatible ends.
And you will need to be able to work with those
in order to figure out whether or not your gene of interest
can ligate into your vector.
Let's complete the process of thinking
about now how to get the gene of interest into the vector, OK?
And the way it goes is that you have
to get your vector ready to receive your gene of interest.
Usually, you cut your vector with the same restriction
enzyme or enzymes that you've cut your gene of interest with.
And then the ends can go together in a matching way.
And you'll get a covalently closed recombinant DNA
molecule that has got both your vector
and your gene of interest.
So you're going to prepare a vector.
And you'll cut it with a restriction enzyme
or restriction enzymes the same as used
to cut the gene of interest.
You then mix together your cut vector
and your cut gene of interest.
And they should have, at this point, compatible ends.
That is your job as a genetic engineer,
to make sure that that's true.
You add DNA ligase to get bonding and a single vector
gene of interest molecule.
And then you take the mix.
You usually have millions and millions of molecules
that you're doing this with.
And you take the whole mix.
And you insert it into the host bacterium, OK?
You insert-- and the correct term is transform.
You insert or transform the whole mix into host bacteria.
And these are the bacteria that that vector likes to grow in.
And the last step in this, then, is that not all the bacteria
are going to get one of these molecules,
these recombinant DNA molecules inserted into them.
In fact, most won't.
It's only a tiny fraction of a percentage that
are going to get a molecule of vector
plus gene of interest inserted.
So you want to get rid of all the bacteria
that don't have your recombinant clone.
And this is where this selectable marker we mentioned
comes in.
You select for bacteria that have got the vector
gene of interest construct.
And usually, the selection is with a particular type
of chemical that is an antibiotic.
And so you put an antibiotic resistance gene
into the plasmid.
And that allows the bacteria that
have got the vector plus the gene of interest
to grow in the presence of antibiotics.
But don't worry about that for now.
But you select for bacteria and the gene of interest.
And then this allows the vector GOI to specifically grow
in the bacteria.
And you can then go ahead and isolate and use the DNA
from this growth mix.
I've drawn this for you in this next slide,
where you can see a gene of interest is cut.
The plasmid vector with its origin of replication is cut.
The two DNAs are ligated.
They've got compatible ends.
And you can actually get three outcomes of this ligation.
You might get your gene of interest just circularizing.
That's not going to be very productive.
Those DNAs will just disappear later in the process.
You might get the vector only that ligates.
That can be a bit of a problem.
And there are ways you can get rid of those.
And then you might get the correct construct,
which is your gene of interest plus the vector.
And that's what you want.
You take that ligation mix, and transform bacteria with it,
and grow, as we said, a lot of the recombinant clone.
The selectable marker comes in because you
can grow your transformants--
the vector or the vector plus gene of interest--
on, in this case, ampicillin, which is an antibiotic.
Normally, ampicillin will stop bacteria from growing.
That's why, if you get a bacterial infection,
antibiotics are the things that you take to treat it.
You can use that.
The bacteria-- we got antibiotics from bacteria.
And now, we can use them in molecular cloning, OK?
So here, there is an ampicillin resistance gene also
on the plasmid vector.
If you grow the bacteria in the presence of ampicillin,
only the bacteria that took up the vector with ampicillin
resistance will be able to grow, OK?
So that's a way to get rid of all the other non-transformed
bacterial clones.
Good.
You've got a lot of information now
about how you put together vectors and inserts, or genes
of interest.
And part of it is the notion of compatible ends.
So I want you to do some practice in this class
exercise, and see if you are able to use the concepts
in a practical way.
Reference Summary
Big Picture: Cloning
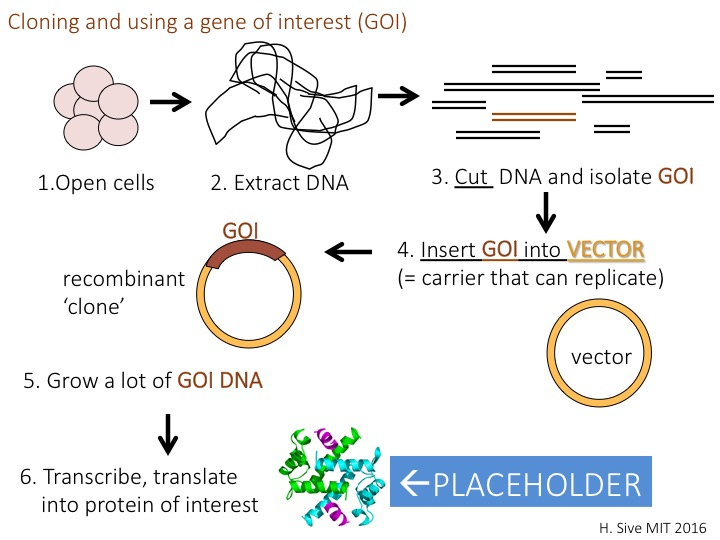
Cloning is the process of isolating a gene of interest (GOI) and expressing it in an organism.
A vector is any carrier of DNA that can deliver that DNA, i.e. the GOI, to the cell and be replicated. One common example of a vector is a plasmid, which is a piece of small, circular DNA.
The cloning process is depicted in detail below.
Restriction Endonucleases: Compatible Ends
Restriction endonucleases, discussed in the previous section, are used to cut out and isolate the GOI (step 3 in the diagram above) and to cut the vector so that the GOI can be integrated into the vector (step 4 in the diagram above).
In order for the GOI to integrate into the vector, the two need to be cut in a way that gives them compatible ends. In this way, they can match up and ligate into a new circular plasmid without any breaks. The different types of compatible ends are detailed below.
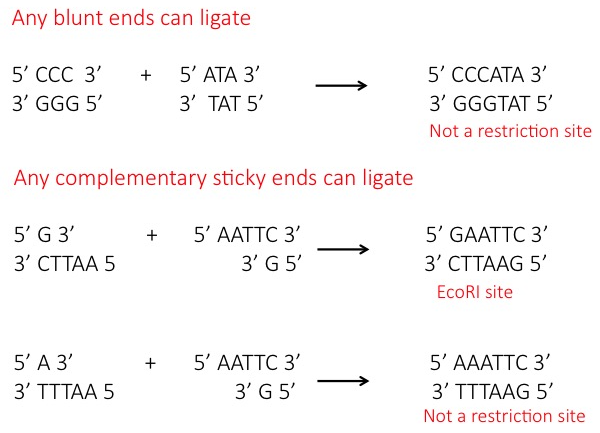
Note that the GOI and the vector do not need to be cut with the same enzyme to be compatible. In the case of blunt ends, all blunt ends can match with other blunt ends. In the case of sticky ends, only the overhanging base pairs need to match up.
However, ligating DNAs from two different restriction sites may prevent the ligation point from serving as a restriction site in the future because you alter the sequence on the other half of the restriction site (in the case of blunt ends) or around the overhanging base pairs (in the case of sticky ends).
Exercise 1 (Blunt Ends)
The following questions concern the two restriction endonucleases shown here.
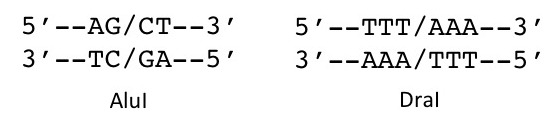
Exercise 2 (Complementary Ends)
The following questions concern the restriction endonucleases shown here.
Exercise 3 (Ligating DNA fragments)
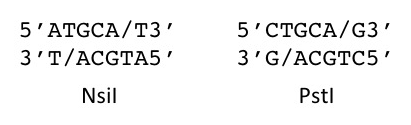
The following questions concern the restriction endonucleases shown here.
MIT OpenCourseWare / MIT Open Learning Library. Hazel Sive and Diviya Ray. Adapted for local study under Creative Commons Attribution–NonCommercial–ShareAlike 4.0. License terms.